Detecting alien newt alleles

In the Netherlands we have a situation where the introduced Italian crested newt is locally replacing the native Northern crested newt. As the Northern crested newt is a threatened species, conservationists would like to try and remove Italian crested newts from the wild. A complication is that the two species hybridize and backcross, resulting in a mix of individuals that are hard to distinguish from natives based on morphology, but that do possess alien alleles. Genetic approaches are required to identify such newts.

ABL

Example for one of the nuclear markers genotyped with our ‘SNPline’ protocol. During PCR two differently fluorescence-labelled tags can be built in, one matching the native allele and the other matching the alien allele. The axes here reflect the level of fluorescence after PCR for each tag. The red cloud reflects individuals with two native copies and the blue cloud individuals with two alien copies, while the green cloud consists of individuals that possess both a native and an invasive allele for this particular marker.

In a previous study we documented the Dutch situation using our Triturus Ion Torrent protocol. The aim of a follow-up study, now published in the journal Conservation Genetics Resources, was to use our existing knowledge on the newt case and design a quick, cheap and easy pipeline to genotype newts on a large scale. Hence, the data required to stop the gradual replacement of the Northern crested newt by the Italian crested newt can now be collected efficiently. Our methodology can also be applied to other cases where the Italian crested newt has been introduced inside the range of the Northern crested newt, known from the UK, Germany and the Swiss/France border.

Reference: Wielstra, B., Burke, T., Butlin, R.K., Schaap, O., Shaffer, H.B., Vrieling, K., Arntzen, J.W. (2016). Efficient screening for ‘genetic pollution’ in an anthropogenic crested newt hybrid zone. Conservation Genetics Resources 8(4): 553-560.

newton_mc
I initiated this work as a Newton International Fellow. This project has received funding from the European Union’s Horizon 2020 research and innovation programme under the Marie Skłodowska-Curie grant agreement No. 655487.
Posted in Uncategorized | 2 Comments

The Anatolian crested newt: a new species endemic to Turkey

11a map

The crested newt traditionally referred to as ‘Triturus karelinii‘ has been split into three species. This map shows their approximate ranges and type localities.

The crested newt species traditionally referred to as ‘Triturus karelinii’ has turned out to be a group of cryptic species. A range-wide mtDNA phylogeography revealed that this taxon comprises three mtDNA clades, as distinct from one another as recognized crested newt species are. To assess the biological meaning of the mtDNA results we subsequently analysed three nuclear DNA markers. The resulting dataset confirmed the existence of three distinct nuclear DNA groups: an eastern, a central and a western one.

There is no evidence for gene flow between the allopatric eastern group and the other two and, based on the type locality, we restricted the name T. karelinii sensu stricto to the eastern group. For the western plus central group the name ‘T. arntzeni’ has previously been used, but at its type locality only newts that show genetic admixture between (predominantly) T. macedonicus and the western group occur. Hence we proposed an alternative name, T. ivanbureschi (sensu lato), in which we placed both the western and central group for the time being.

image description

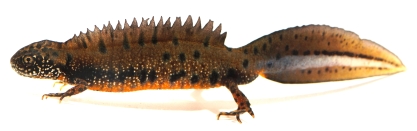
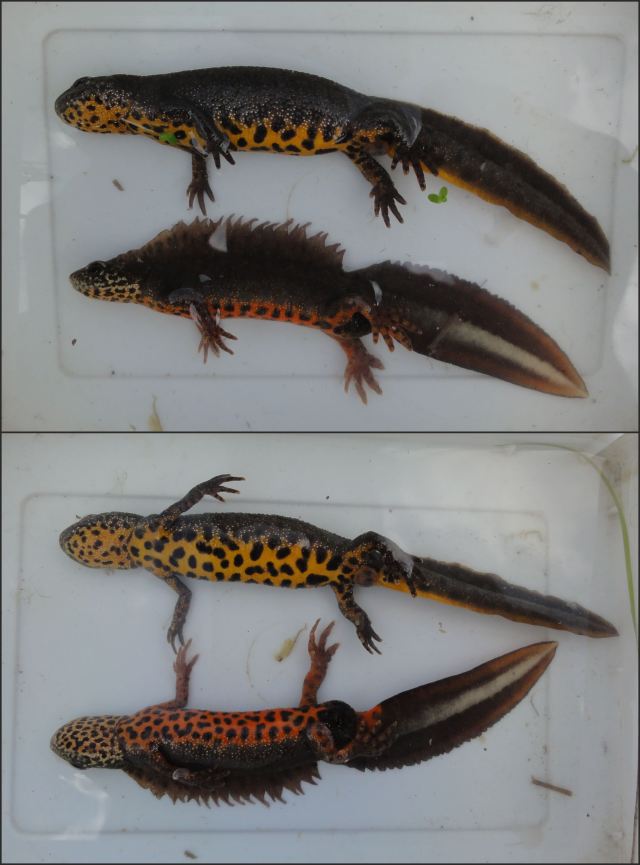
These sedated newts, a female above and a male below, are from the type locality of Triturus anatolicus.

The taxonomical question of whether the two groups comprising T. ivanbureschi sensu lato are different species remained. As the two occur in parapatry and show evidence of at least some recent gene flow, we preferred not to jump to conclusions. We first conducted a detailed hybrid zone analysis with the aid of the Triturus Ion Torrent protocol. Although not the main aim of the hybrid zone study (to be published separately) we could use the data to determine if the two groups comprising T. ivanbureschi should be regarded as distinct species. We could confirm that both groups comprising T. ivanbureschi sensu lato manage to maintain their genetic integrity. Because the type locality is positioned in the range of the western group, the name of T. ivanbureschi should be restricted to that group. We have now described the central group as a distinct species, dubbed T. anatolicus, in the journal Zootaxa. Up to now only genetic data have been used to identify the three crested newt species comprising the T. karelinii sensu lato group. The next step is to take a better look at these newts and see if morphological features that separate the species can be discovered.

11c type locality

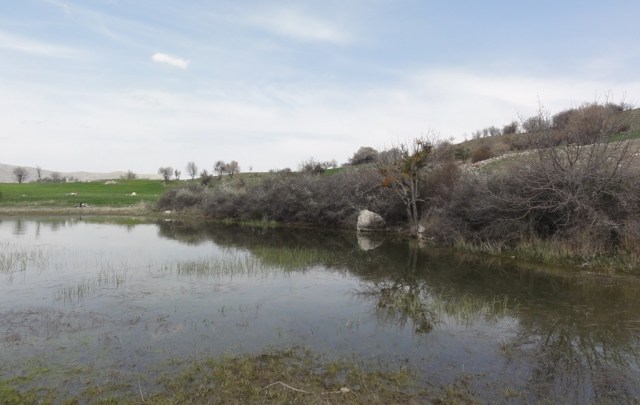
This pond is the type locality of Triturus anatolicus.

Reference: Wielstra, B., Arntzen, J.W. (2016). Description of a new species of crested newt, previously subsumed in Triturus ivanbureschi (Amphibia: Caudata: Salamandridae). Zootaxa 4109(1): 073-080.

newton_mc
I initiated this work as a Newton International Fellow. This project has received funding from the European Union’s Horizon 2020 research and innovation programme under the Marie Skłodowska-Curie grant agreement No. 655487.
Posted in Uncategorized | 1 Comment

No subspecies for the Danube crested newt

T.dobrogicus_Danube DeltaMale T. dobrogicus. Picture by Michael Fahrbach.

The taxonomical history of Triturus has been (and is) a turbulent one. However, genetic data has been very helpful in clearing it up. After our recent taxonomical revision of the genus, all species in the genus were considered monotypic except for one: in the Danube crested newt (T. dobrogicus) two subspecies were still recognized. But was this justified? No strong evidence was published in favour and recent work in fact seemed to disagree with this treatment. To settle the matter once and for all we turned to the power of the Triturus Ion Torrent protocol. After testing for the presence of intraspecific genetic structuring we could only conclude that there was none, or at least none that would fit the two subspecies hypothesis. Hence, in a recent paper in Amphibia-Reptilia, we suggest to treat the Danube crested newt as monotypic as well. Nice and tidy.

Reference: Wielstra, B., Vörös, J., Arntzen, J.W. (2016). Is the Danube crested newt Triturus dobrogicus polytypic? A review and new nuclear DNA data. Amphibia-Reptilia 37(2): 167-177.

newton-logo

I conducted this work as a Newton International Fellow.
Posted in Uncategorized | Leave a comment

Genetic pollution in Dutch crested newts

Invasive species threaten native biota, not only through competition, predation and infection, but also via hybridization. Human-induced hybridization has important implications from the point of view of conservation as it results in genetic replacement – a loss of biodiversity at the level of the gene. However, because hybridizing species are often closely related and morphologically similar, ‘genetic pollution’ is insidious. To expose and quantify genetic pollution, genetic data need to be consulted.

In several localities within the range of the threatened Northern crested newt (Triturus cristatus), the Italian crested newt (T. carnifex) has been introduced. In the Netherlands T. carnifex has established itself on the Veluwe and poses a potential threat there to the native T. cristatus. At the request of the Invasive Alien Species Team,  my MSc. student Willem Meilink and I, in collaboration with the Dutch NGO RAVON (Reptile, Amphibian and Fish Conservation Netherlands), used the new Triturus Ion Torrent protocol to explore the issue of genetic pollution of T. cristatus by T. carnifex. We recently published a paper in Biological Conservation on the case. Populations vary from completely invasive, via different degrees of genetic admixture, to completely native, when sampling outwards from the initial site of introduction of the exotic species. The observed pattern shows that the two crested newt species are hybridizing on the Veluwe and that the exotic T. carnifex is expanding at the expense of the native T. cristatus.
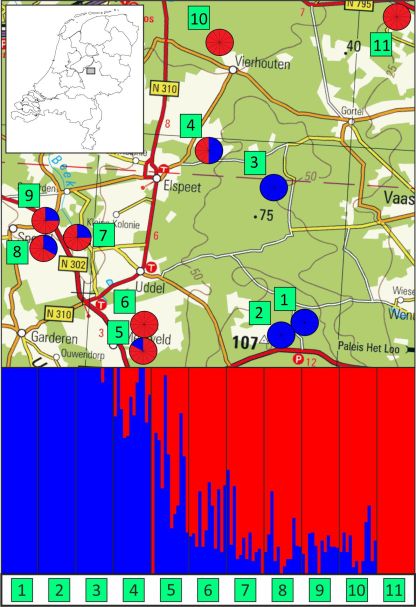
This figure shows the study area with eleven studied ponds (above) and the genetic composition of twelve individuals sampled for each pond (below). From pond 1 to 11 the proportion of genetic material of the invasive T. carnifex (blue) decreases, whereas that of the native, threatened T. cristatus (red) increases. The top panel also shows the distribution of mitochondrial DNA in the ponds (using the same color scheme); note that it underestimates the spread of T. carnifex.

This figure shows the study area with eleven studied ponds (above) and the genetic composition of twelve individuals sampled for each pond (below). From pond 1 to 11 the proportion of genetic material of the invasive T. carnifex (blue) decreases, whereas that of the native, threatened T. cristatus (red) increases. The top panel also shows the distribution of mitochondrial DNA in the ponds (using the same color scheme); note that it underestimates the spread of T. carnifex.

Our study shows that the invasive species poses a threat to the native species through genetic pollution. However, countering this threat, if one would decide to do so, is far from straightforward. Which individuals deserve protection? How to deal with individuals with an almost native genotype? What is the legal status of such individuals? Even when you have made a decision, how will you establish in practice whether a particular individual meets your requirement? Are there instances where you should consider maintaining genetic integrity of the native species infeasible? What if most individuals have become polluted? Tackling these dilemmas requires interaction between scientists, conservationists, legislators and land managers. We hope this case study will help drafting as yet non-existent guidelines for the management of genetic pollution.

This study was funded by the Invasive Alien Species Team, which advices the Ministry of Economic Affairs on the management of invasive species, and it was conducted in collaboration with the Dutch NGO RAVON (Reptile, Amphibian and Fish Conservation Netherlands), responsible for monitoring amphibians (and reptiles and fish) in the Netherlands.

Reference: Meilink, W.R.M., Arntzen, J.W., van Delft, J.C.W., Wielstra, B. (2015) Genetic contamination of a native threatened crested newt species through hybridization with an invasive congener. Biological Conservation 184: 145-153.

Reference: Wielstra, B., Arntzen, P., van Delft, J., Meilink, W. (2015). Genetische vervuiling op de Veluwe: hybridisatie tussen een inheemse en een exotische kamsalamandersoort. RAVON 17(2): 36-39.

Reference: Meilink, W.R.M., Arntzen, J.W., Wielstra, B. (2013). Genetische vervuiling op de Veluwe: Hybridisatie tussen de inheemse Noordelijke kamsalamander en de invasieve exoot Italiaanse kamsalamander. Naturalis Biodiversity Center, Leiden.
newton-logo

I conducted this work as a Newton International Fellow.
Posted in Uncategorized | 5 Comments

Two notes on the Kosswig’s newt

Last spring Emin Bozkurt and I were conducting fieldwork in Turkey. Although we were specifically targeting crested newts, we came across many Lissotriton newts as well. We were quite surprised to catch some paedomorphic Kosswig’s newts (Lissotriton kosswigi). Paedomorphism is the retention by adults of traits normally seen only in juveniles. In newts this constitutes keeping the gills into adulthood and having a fully aquatic lifestyle rather than spending a chunk of the year on land. It is not unexpected that paedomorphism occurs in the Kosswig’s newt, considering that paedomorphism has been reported for most of the Kosswig’s newts cousins, but paedomorphic Kosswig’s newts had never been documented before. Hence, we published a note in the Turkish Journal of Zoology about our encounter.

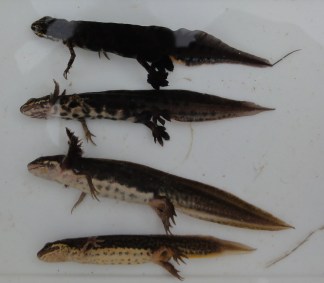
9aFrom top to bottom these are a normal adult male, a paedomorphic male, a paedomorphic female and a normal adult female Kosswig’s newt. Notice the gills of the paedomorphs. The male shows a swollen cloaca, meaning it is sexually mature and hence an adult.

Reference: Bozkurt, E., Olgun, K., Wielstra, B. (2015). First record of facultative paedomorphism in the Kosswig’s newt Lissotriton (vulgaris) kosswigi (Freytag, 1955) (Urodela; Salamandridae), endemic to northwestern Turkey. Turkish Journal of Zoology 39: 976-980.

The Kosswig’s newt and its Turkish congener the Schmidtler’s newt have always fascinated me. The reason for this is that they show a similar biogeographical pattern to crested newts. For both groups of newt a relatively recent shift of distribution ranges, in response to a re-arrangement of the marine connection between the Black and Marmara Seas, is strongly suspected. The advantage of the Lissotriton newts is that they are morphologically quite distinct, whereas for crested newts we (as yet) have to rely on genetics for species identification. On top of the comparative biogeographical pattern, the Kosswig’s newt has a very limited distribution range and its species status is not generally accepted. In this context we wrote a paper on the distribution and taxonomy of all the Turkish Lissotriton newts for Zookeys.

The Kosswig’s (top) and Schmidtler’s newt are quite different. The crest is smooth and starts above the forelimbs in the Kosswig’s newt and is ragged and starts in the neck in Schmidtler’s newt. The Kosswig’s also differs from the Schmidtler’s newt in having a threadlike tail filament and very flappy feet.

Reference: Wielstra, B., Bozkurt, E., Olgun, K. (2015). The distribution and taxonomy of Lissotriton newts (Amphibia, Salamandridae) in Turkey. ZooKeys 484: 11-23.

Please note that newts normally do not pose for pictures like the ones above; these newts were temporally sedated.

newton-logo

I conducted this work as a Newton International Fellow.
Posted in Uncategorized | 3 Comments

A crested newt refugium in the Carpathians

The current Pleistocene Ice Age has heavily influenced the distribution of species. One could argue it still does – the Ice Age is not a thing of the past, we are now merely experiencing a relatively warm interval (called the Holocene). During an Ice Age, the climate cycles between long cold spells (glacial periods) and short warm spells (interglacials) and this temperature fluctuation is larger, further away from the equator. During the glacial periods many species had their ranges reduced in so-called glacial refugia, where conditions remained agreeable (whereas populations outside these areas went extinct). During interglacials they could expand their distributions again from these glacial refugia. This pattern of range reduction and expansion repeated itself with each climate cycle.

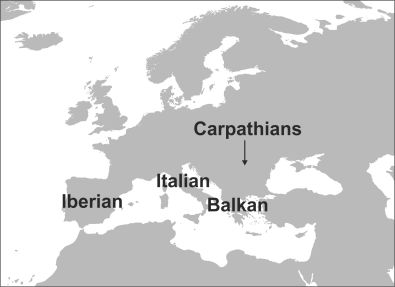
The three southern European peninsulas – Iberian, Italian and Balkan – played a major part as glacial refugia. Many temperate species had their ranges reduced to one of these peninsulas during glacial periods and colonized the rest of their European from here as glacial conditions alleviated. The Carpathians are now increasingly being recognized as a relatively northern glacial refugium.

The three southern European peninsulas – Iberian, Italian and Balkan – played a major part as glacial refugia. Many temperate species in Europe had their current ranges reduced to one of these peninsulas during glacial periods and they colonized the rest of their current range from here as glacial conditions alleviated. The Carpathians are now increasingly being recognized as a relatively northern glacial refugium.

In stable populations in glacial refugia genetic diversity accumulates over time and, when they get isolated from one another, such populations diverge. On the other hand, postglacially established populations typically arise from a few founders that represent only a fraction of the total genetic variation present in a species. Hence, population stability and expansion leave different signatures in a species’ genes across its range. The late Godfrey Hewitt, thinking from a northern hemisphere perspective, dubbed this pattern “southern richness and northern purity”.

The genetic diversity for T. cristatus is high in the Carpathian region (two lower panels; mitochondrial DNA (left) and nuclear DNA show three main genetic groups, populations in grey are genetically admixed with other crested newt species). However, genetic diversity is basically zero in the rest of its range (top panel; one genetic group only). In the lower panels the Carpathian mountain range is shaded grey.

The genetic diversity for T. cristatus is high in the Carpathian region (two lower panels; mitochondrial DNA (left) and nuclear DNA show three main genetic groups, represented by different colors; populations in grey are genetically admixed with other crested newt species). However, genetic diversity is basically zero in the rest of its range (top panel; one genetic group only). In the lower panels the Carpathian mountain range is shaded grey.

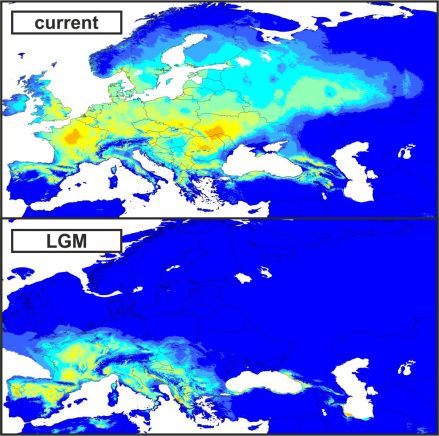
As we strongly suspected that the crested newt Triturus cristatus provides a particularly extreme example of the “southern richness and northern purity” paradigm, we conducted a detailed screening of genetic diversity and investigated the distribution of suitable habitat at the height of the last glaciation. Several distinct genetic clusters occur in the Carpathians nowadays, whereas in the rest of its range T. cristatus shows extreme genetic depletion: newts from the UK and the Urals are indistinguishable based on the markers we studied! Most of the current range of T. cristatus was totally uninhabitable at the Last Glacial Maximum, but suitable area remained in the Carpathians. Our study, published in the Biological Journal of the Linnean Society, shows that most of the huge current range of T. cristatus was only colonized after the last glacial period ended, from a glacial refugium situated in the Carpathian region.

These ecological niche models show area predicted suitable for T. cristatus nowadays (top) and at the height of the last glacial period, the Last Glacial Maximum (c. 21,000 years ago).

These ecological niche models show area predicted suitable for T. cristatus nowadays (top) and at the height of the last glacial period, the Last Glacial Maximum (c. 21,000 years ago).

Reference: Wielstra B, Babik W, Arntzen JW (2015). Postglacial recolonization of Europe by the crested newt Triturus cristatus from an extra-Mediterranean glacial refugium – the Carpathian region. Biological Journal of the Linnean Society 114(3): 574-587.

newton-logo

I conducted this work as a Newton International Fellow.
Continue reading

Posted in Uncategorized | 12 Comments

Marie Skłodowska-Curie Fellowship

I have been awarded an ‘outgoing’ Marie Skłodowska-Curie Fellowship. This will allow me to visit the lab of Brad Shaffer at the University of California, Los Angeles in the USA to learn sequence capture by target enrichment for two years. My third ‘return’ year will be back at the University of Sheffield, in the lab of Roger Butlin.

MSCactions

Posted in Uncategorized | Leave a comment

Trying to crack the crested newt phylogeny – and failing

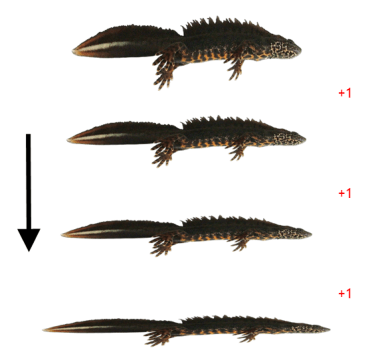
The four main groups of crested newt species differ in body shape. This morphological variation is correlated with ecological differences: sturdier newts are more terrestrial and slenderer newts more aquatic. This suggests that the differentiation in body shape drove their evolution and that gradually more and more slender newts evolved (by looking at related newts we can deduce that the ‘ancestral’ crested newt was stocky). Conveniently, body shape variation is reflected by discrete differences in the number of rib-bearing vertebrae, with each additional rib corresponding to a slightly more stretched body shape.

6a elongation

The hypothesis is that the radiation of Triturus body shapes came about by stepwise elongation (expressed by the evolution of additional ribs).

However, the crested newts represent a rapid radiation: the four main groups originated in a relatively short time span. This makes it particularly difficult to resolve the relationships between the groups. Previously, using full mitochondrial genomes, we managed to get a resolved tree. However, the mitochondrial genome behaves as a single gene and hence a single estimate of evolutionary history. The nuclear genome, on the other hand, provides a much deeper understanding.

The branching order in Triturus based on full mitochondrial genomes is fully in line with a scenario of body shape evolution involving the least possible evolutionary steps required (here expressed as additions of rib-bearing vertebrae). I dare you to you can find a tree that explains the variation in the number of ribs requiring less steps.

The branching order in Triturus based on full mitochondrial genomes is fully in line with a scenario of body shape evolution involving the least possible evolutionary steps required (here expressed as additions of rib-bearing vertebrae). I dare you to find a tree that explains the variation in the number of ribs in less steps.

Wouldn’t it be great if we could confirm the mitochondrial tree using a battery of nuclear genes? With this mission in mind I used an adaptation of my Ion Torrent protocol to collect relatively long genes with 454 next-generation sequencing. Without going into details, let me tell you it was a huge effort to collect the dataset. But now surely we would solve the crested newt relationships once and for all right? Right?

The new Triturus tree based on an order of magnitude more nuclear genes than previously studied is a mess. There is no support for any particular branching order and provides no insight into the evolution of the number of ribs at all.

The new Triturus tree, based on an order of magnitude more nuclear genes than previously studied, is a mess. There is no support for any particular branching order and the tree provides no insight into the evolution of the number of ribs at all.

Not a chance. After finally getting the computationally super heavy analyses to run properly (and waiting a considerable time for them to finish) results were disappointing. Even with all these data and an array of analytical approaches, we could not resolve the evolutionary tree of the crested newts. However, this is a biological reality: our study, published in PLoS ONE, illustrates perfectly the difficulty of resolving rapid radiations. The crested newts are a particularly suitable system to explore the matter further, but for this we need to wait until genome-scale data are available.

Reference: Wielstra, B., Arntzen, J.W., van der Gaag, K., Pabijan, M., Babik, W. (2014). Data concatenation, Bayesian concordance and coalescent-based analyses of the species tree for the rapid radiation of Triturus newts. PLoS ONE 9(10): e111011.

newton-logo

I conducted this work as a Newton International Fellow.
Posted in Uncategorized | 7 Comments

NWO ALW Open grant

A grant proposal I wrote together with Pim Arntzen was successful and will allow us to hire a PhD student to work on amphibian hybrid zones.

nwo-logo

Posted in Uncategorized | Leave a comment

Mapping the European Triturus species

In 2014 the New Atlas of Amphibians and Reptiles of Europe (the first update since 1997’s original atlas) was published in the journal Amphibia-Reptilia. In the new atlas, the crested newts and marbled newts were mapped as such, even though both of these two groups encompass more than one species. However, as these species are morphologically similar and, on top of that, hybridize at their poorly documented contact zones, the authors of the new atlas did not feel they could confidently map their distributions. We are working extensively on these newts and, particularly based on our recent field trips and our new Triturus Ion Torrent protocol, have accumulated enough data to allow us to map the individual species. Hence, in a follow-up paper in Amphibia-Reptilia, we published distribution maps of all the species that comprise the marbled and the crested newt groups.

This is an overview of all the European grid cells that have Triturus localities (with cells having more than one species coloured blue rather than red). Maps for the individual species are published with the paper.

This is an overview of all the European grid cells that have Triturus localities (with cells having more than one species coloured blue rather than red). Maps for the individual species are published with the paper.

Reference: Wielstra, B., Sillero, N., Vörös, J., Arntzen, J.W. (2014). The distribution of the crested and marbled newt species (Amphibia: Salamandridae: Triturus) – an addition to the New Atlas of Amphibians and Reptiles of Europe. Amphibia-Reptilia 35(3): 376 –381.

newton-logo

I conducted this work as a Newton International Fellow.
Posted in Newts | 1 Comment